The Promise and Peril of Self-Sustaining Genetic Intervention
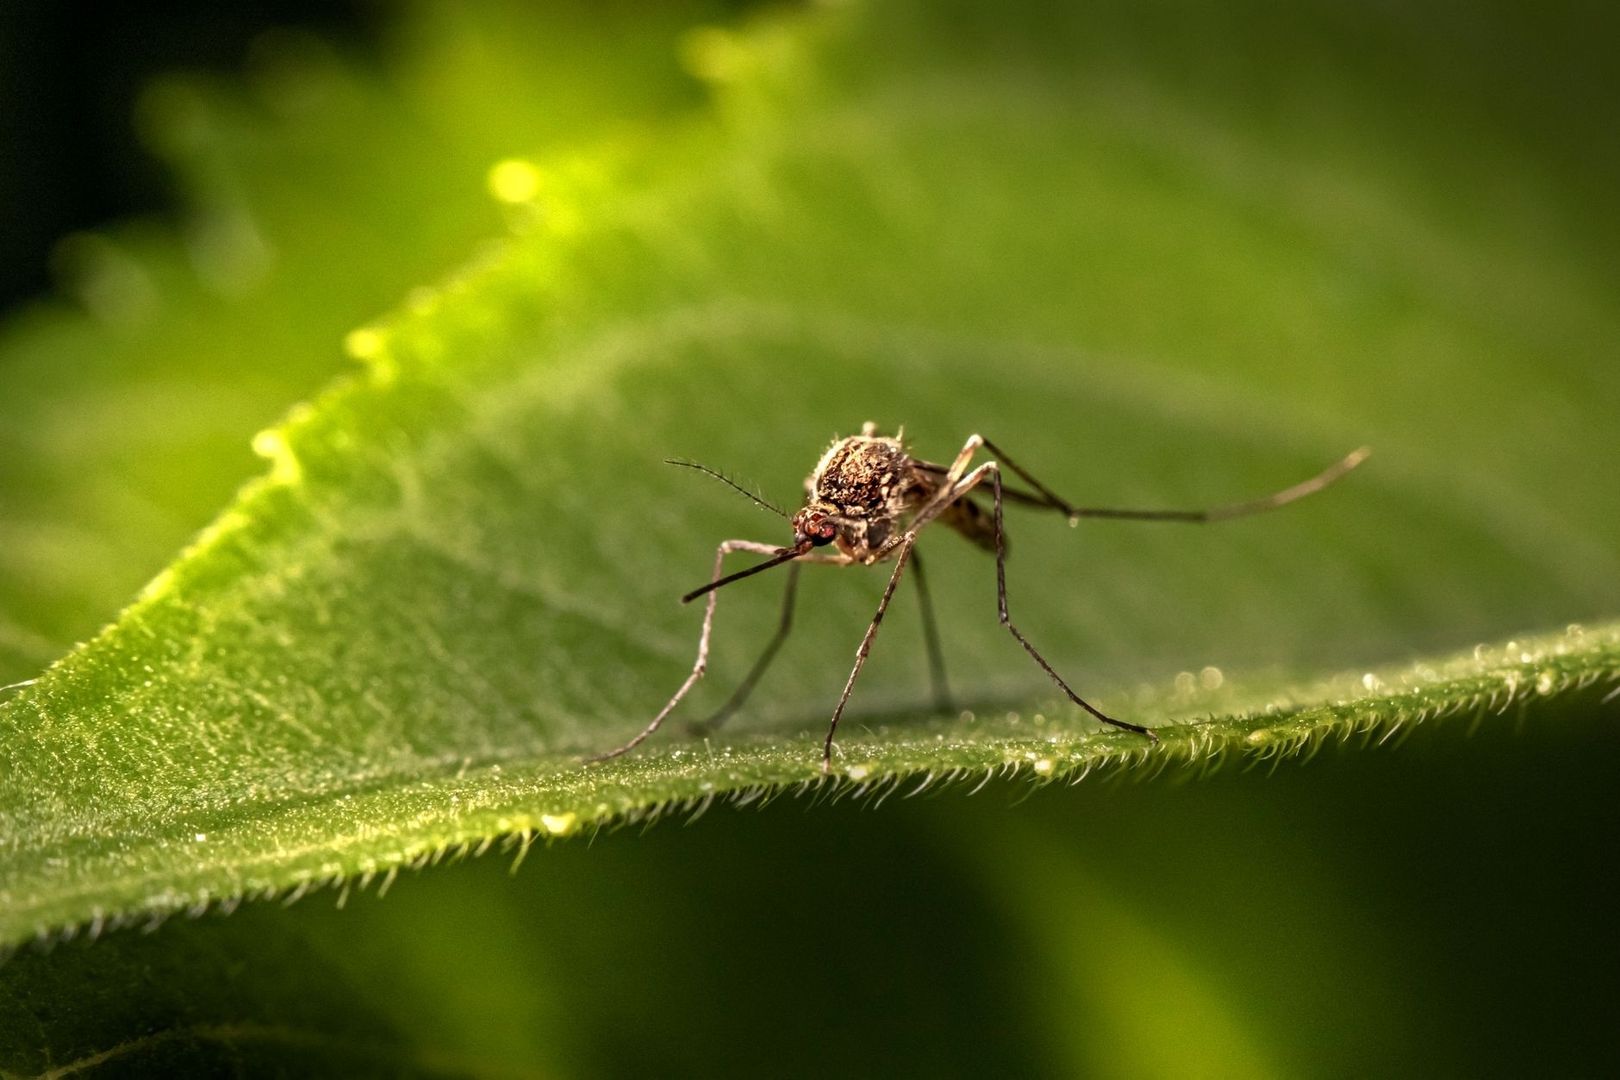
Conventional genetically modified organisms are generally designed to remain within a managed production or research system. A CRISPR gene drive is different in kind, not merely degree. It is engineered to alter the ordinary rules of inheritance so that a chosen genetic sequence spreads through a wild population more efficiently than Mendelian genetics would normally allow. The ambition is substantial: suppress a disease-carrying insect, replace a harmful trait, or remove an invasive population without repeated chemical treatment or continual release programmes.
That ambition also changes the meaning of containment. A laboratory can use physical barriers, controlled breeding, quarantine procedures and genetic safeguards. An open ecosystem has none of these protections in a reliable, comprehensive form. Animals move across landscapes, wind carries insects, borders divide habitats rather than species, and related organisms may exchange genes. The distinction between a contained experiment and an environmental intervention is therefore fundamental. Once a self-sustaining drive enters a connected population, control depends on ecological assumptions that may prove wrong over decades.
The central biosecurity paradox is stark. The very feature that makes a gene drive attractive is its resistance to dilution. It is intended to persist, spread and overcome the ordinary tendency of introduced genes to disappear through breeding. Yet if an unforeseen consequence emerges, that same persistence becomes the problem. There is no biological equivalent of recalling a defective product from every field, forest or wetland. A technology designed never to be naturally purged cannot be treated as though it will politely remain within the boundaries of the original decision.
Mendel Overruled How Gene Drives Alter Population Dynamics
Under ordinary Mendelian inheritance, an individual carrying one altered version of a gene and one natural version typically passes either version to offspring. A heterozygote therefore transmits the altered allele to roughly half its descendants, subject to selection, mating patterns and chance. A homing gene drive uses CRISPR-associated molecular machinery to cut the matching natural chromosome in the germline. If the cell repairs that break using the drive-bearing chromosome as a template, the engineered sequence can be copied into the cut site. The former heterozygote is converted, in effect, into an individual carrying two drive copies.
This process can raise inheritance well above the expected 50 percent and, under favourable laboratory conditions, towards near-total transmission. That does not mean every release will spread indefinitely. Fitness costs, resistant mutations, population structure, sex-specific effects, mating behaviour and environmental conditions all matter. Research on natural-population dynamics shows why simple laboratory models can mislead: density dependence, spatial variation and movement between subpopulations may determine whether a drive expands, stalls, fragments or selects for resistance. The evidence base remains strongest for controlled or highly managed settings, not for the full complexity of wild ecosystems.
Two broad purposes are often confused in public debate. A suppression drive seeks to reduce reproduction or skew the sex ratio until a target population declines sharply, potentially approaching local eradication. A replacement drive seeks to leave population numbers broadly intact while spreading a trait, such as reduced ability to transmit a pathogen. These aims carry different ecological and ethical questions. Removing a species from one landscape may alter predators, competitors and food webs, while replacing a trait may create a persistent genetic change whose wider effects are difficult to anticipate. Foundational explanations of non-Mendelian inheritance, including those collected by the National Academies and biomedical repositories, make clear that gene drives are designed to force population-level genetic shifts rather than follow ordinary inheritance.
- Classic Mendelian inheritance: a heterozygous individual commonly passes an allele to about 50 percent of offspring.
- Active gene drive inheritance: CRISPR cutting and template-based repair can copy the drive into the matching chromosome, producing transmission substantially above 50 percent.
- Ordinary genetic dilution: introduced traits may decline when they impose a fitness cost or when carriers mate with unmodified individuals.
- Self-sustaining drive behaviour: the construct is intended to spread from relatively low frequency, although resistance and ecological conditions can interrupt that spread.
- Suppression strategy: reduce fertility, survival or the production of one sex to lower population abundance.
- Replacement strategy: spread a trait that changes population function, such as the ability to transmit a pathogen, without necessarily reducing abundance.
The Engineering Myth of Reversal Drives and Biological Recall
Proposals for genetic recall often sound more reassuring than they are. An immunising drive might overwrite an earlier drive or make future generations resistant to it. A reversal drive might introduce a sequence intended to restore the original genetic state. Split-drive designs separate essential components so that the system becomes dependent on repeated releases, while a secondary Cas9 construct could, in theory, target and disable an earlier intervention. These are valuable research concepts, but they are not equivalent to a proven off switch.
Every secondary intervention must itself spread through the population, find the relevant genetic sequence and remain functional across diverse genomes and changing environments. The first drive may already have generated cleavage-resistant alleles through error-prone repair. Guide RNA target sites may mutate, be deleted or differ between populations. Cas9 activity may create unintended edits, while the reversal construct may carry its own fitness cost and fail to reach enough individuals. A rescue strategy that works in a laboratory strain may be ineffective against wild genetic diversity, seasonal population turnover or migration from an untreated area.
The broader containment literature reinforces the point. Biological safeguards such as auxotrophy, kill switches, toxin-antitoxin systems and environmentally responsive circuits can reduce escape probabilities, but individual mechanisms may be bypassed, reverted or undermined by horizontal gene transfer. Layered systems can improve performance, yet they require long-term stability and continuous verification. Peer-reviewed work on evolutionary escape routes in genomic safeguards illustrates why intended synthetic controls must be assessed against mutation, selection and ecological exposure rather than only their initial laboratory performance.
In an open biome, genetic material cannot simply be vacuumed back into a sterile laboratory. A recall release would be another ecological intervention, with its own dispersal pattern, evolutionary trajectory and possible effects on non-target organisms. It might reduce the original construct in one population while selecting for resistant variants in another. The responsible question is therefore not whether a reversal design can be imagined, but whether it has demonstrated reliable, species-wide, multi-generational control under realistic conditions. At present, that standard has not been met for an open, self-sustaining extinction-level drive.
| Proposed safeguard | Intended function | Operational vulnerability |
|---|---|---|
| Split drive | Separate essential components to limit persistence | Components may recombine, persist longer than expected, or behave differently in wild populations |
| Immunising drive | Make organisms resistant to a prior drive | Requires efficient spread and accurate recognition of all relevant drive variants |
| Reversal drive | Overwrite or remove an earlier genetic construct | Target-site resistance, incomplete conversion and new fitness costs may block recall |
| Secondary Cas9 system | Cut and disable the original sequence | Off-target edits, guide RNA breakdown and genetic diversity can reduce effectiveness |
| Kill switch or auxotrophy | Make survival dependent on a controlled condition | Mutation, environmental substitutes and horizontal transfer can undermine containment |
Borders on the Map Versus Species in the Wind
Gene drives create a direct governance problem because biological movement does not follow sovereign consent. A mosquito, rodent or insect carrying a drive may cross a national border without any formal transfer, permit or diplomatic notification. A country that declines a release could still face exposure through migration, trade pathways or connected habitat. The ethical issue is not confined to whether the technology is beneficial in the releasing state. It includes whether neighbouring populations have a meaningful right to refuse an intervention that may alter their ecosystems permanently.
Non-target effects are also more complicated than a simple question of whether CRISPR cuts the intended gene. Closely related species may hybridise, allowing genetic material to move beyond the target. Horizontal gene transfer is less predictable but remains relevant to the assessment of engineered sequences, particularly where microbial communities, parasites or mobile genetic elements are involved. Changes in abundance can then propagate through food webs. Predators may lose prey, competitors may expand, disease transmission may shift, and ecological functions may change even when the molecular edit appears precise.
The Convention on Biological Diversity and the Cartagena Protocol provide important principles and information-sharing mechanisms, including the Biosafety Clearing-House, but they were not designed as a complete international recall system for self-sustaining gene drives. The Kunming-Montreal Global Biodiversity Framework, adopted in 2022, recognises biosafety and the potential benefits of biotechnology through Target 17. That recognition must not be mistaken for blanket permission. Reviews of international synthetic-biology policy, including developments discussed through the biodiversity process and the 2024 negotiations, show a framework still evolving rather than a settled protocol for transboundary gene-drive deployment.
- Prior informed consent should cover potentially affected states, not only the jurisdiction hosting a release.
- Risk assessment should examine related species, migration corridors, food webs and genetic diversity across the entire plausible range.
- Public participation should include Indigenous peoples, local communities, farmers, conservation bodies and neighbouring governments.
- International data sharing should include release plans, genetic sequences, monitoring results and evidence of resistance or spread.
- Disagreement should trigger pause and review, not be treated as a procedural inconvenience.
Closing the Biosafety Governance Deficit
Standard market biosafety testing is usually designed around a product, a use case and a defined period of assessment. Autonomous gene drives require something more demanding: long-term evolutionary stewardship. Regulators must ask not only whether the organism performs its intended function, but also how the construct may mutate, persist, recombine, move between populations and interact with ecological change. The relevant time horizon is not a commercial launch cycle. It is the life of the affected population and the persistence of the genetic intervention.
Governance must also be broader than a technical approval issued by a single agency. Existing proposals emphasise accountability, transparency, participation, uncertainty analysis and adaptive oversight. The CBD”s information systems, including the Biosafety Clearing-House resources, can support cooperation, but information exchange is not the same as enforceable accountability. Communities need access to the evidence, independent experts must be able to challenge risk assessments, and regulators must retain the power to halt experiments when monitoring reveals unexpected spread.
A responsible framework would require at least the following sequence before any open-air field test could be contemplated:
- Define the ecological objective precisely. The applicant should demonstrate why a gene drive is necessary, identify less persistent alternatives and explain who bears the risks and who receives the benefits.
- Characterise the target and its relatives. Testing should cover wild genetic diversity, mating barriers, hybridisation potential, geographic range and relevant food-web relationships.
- Demonstrate layered containment. Physical, reproductive, molecular and ecological safeguards should operate independently, with multi-generational testing rather than short laboratory trials.
- Model realistic failure. Assessments should include resistance, off-target changes, guide RNA degradation, migration, recombination, climate-driven range shifts and incomplete recall.
- Secure transboundary consent. Potentially affected jurisdictions should have access to data, independent review and a genuine veto before release.
- Fund independent monitoring. Surveillance should continue for decades, with agreed indicators, public reporting and resources guaranteed before release rather than sought after an incident.
- Establish liability and remediation. Developers and authorising states should contribute to a financial mechanism capable of supporting affected communities, ecological restoration and emergency research.
The Kunming-Montreal framework can provide a political foundation, but Target 17 should not be used as a shortcut around precaution. Binding international rules would need to clarify responsibility when a drive crosses borders, including who pays for monitoring and who has authority to order further intervention. A sovereign veto, transparent evidence standards and a liability fund would not prevent beneficial research. They would establish the minimum conditions under which public trust could be earned. Without them, the costs of a failure may fall on communities and ecosystems that had no role in the original decision.
Demanding Precaution Before Erasing the Rewind Button
The engineering gap is now clear. Synthetic biology can design powerful inheritance systems, but biological evolution remains more variable, opportunistic and geographically expansive than any laboratory safeguard. A drive may mutate, encounter resistant alleles, move into a related population or behave differently under real ecological pressures. A proposed reversal mechanism faces the same evolutionary forces as the original intervention, and perhaps a more difficult task because it must find and neutralise what has already spread.
Treating an entire ecosystem as a testbed without an absolute recall capability converts scientific optimism into an irreversible ecological gamble. Gene drives may eventually offer public-health or conservation benefits, but those claims must be scrutinised against the evidence, not accepted on the strength of theoretical models or commercial urgency. Independent oversight, strict precaution, transparent monitoring and binding international accountability should come before open release. Scientific honesty requires stating plainly what current technology cannot promise: once an extinction-level drive is released into a connected wild population, there may be no rewind button.